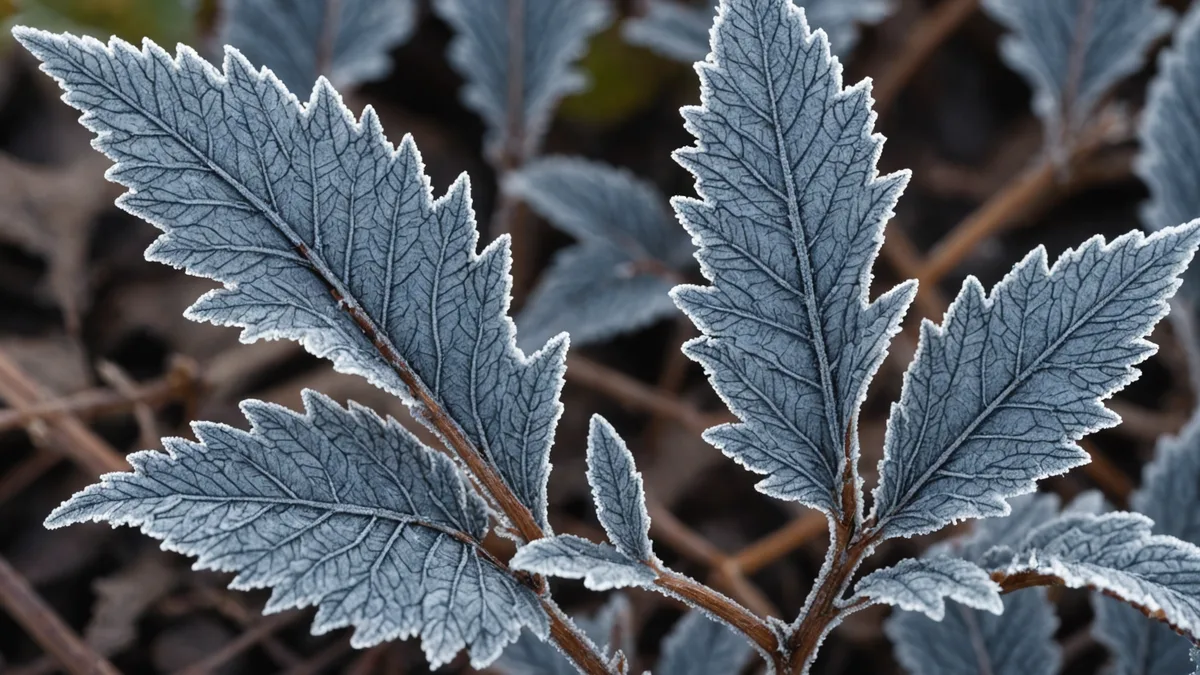
Late-frost events in Patagonian growing regions follow a pattern that growers know well but that has not consistently attracted the same policy and research attention as drought or salinization. The temperature swings are extreme: air temperatures in spring can drop to -4C or lower during a clear radiation frost night after several weeks of warm days that have pushed seedling development past the tolerance threshold for that crop. When maize or potato seedlings have already developed two to three leaf pairs, a single sharp frost event can kill the shoot tips and wipe out stand establishment entirely.
Climate projections for southern South America suggest this pattern of irregular frost timing is likely to intensify rather than diminish: warmer average temperatures bring earlier emergence and development, but the window for late frost events remains open or expands due to increased inter-annual variability. The practical agricultural problem is that the risk window when crops are most vulnerable overlaps increasingly with the planting window.
What Frost Actually Does to Plant Cells
Cold stress in plants encompasses two distinct physiological problems: chilling injury, which occurs above freezing when metabolic processes are disrupted by cold temperatures, and freezing injury, which occurs when extracellular ice crystals form and mechanically damage cell membranes. Late-frost events in Patagonian spring conditions involve both, often in the same 12-hour period as temperatures drop from above-zero in the afternoon to sub-zero at 4 AM and recover again by morning.
Extracellular ice crystal formation is the more immediately lethal mechanism. Ice crystals form preferentially in extracellular spaces because solute concentrations there are lower and nucleation temperatures are higher. As extracellular water freezes, the osmotic gradient pulls water out of adjacent cells, causing cellular dehydration. If the dehydration is severe and the temperature drop is fast enough that rewarming cannot allow membrane repair, cells die. The leaf tip browning and wilting that growers see the morning after a sharp frost is this process made visible.
Chilling injury is slower but cumulative. Cold temperatures shift the phase transition behavior of membrane lipids, increasing membrane rigidity and disrupting the membrane-bound enzyme complexes involved in photosynthesis, particularly Photosystem II. Crops with high proportions of saturated fatty acids in their membrane lipids are more vulnerable to this transition; conversely, organisms adapted to cold environments typically maintain membrane fluidity at low temperature by upregulating fatty acid desaturase enzymes that increase the proportion of unsaturated fatty acids.
Psychrotolerant Bacteria and the Cold-Shock Response
Psychrotolerant and psychrophilic bacteria that live in cold Patagonian soils year-round have evolved a toolkit for surviving exactly these conditions. Their cold-shock mechanisms include several pathways that are relevant to our screening work.
Cold-shock proteins of the CspA family are small RNA chaperones that prevent the formation of inhibitory secondary structures in mRNA at low temperatures. When a bacterium experiences a rapid drop in temperature, CspA-family proteins are among the first genes induced, stabilizing transcripts that would otherwise form hairpin structures blocking ribosome binding. This is a common mechanism across bacterial cold-adaptation, but the diversity of CspA homologs in Patagonian isolates from highly variable temperature environments is notable: strains sampled from frost-prone volcanic steppe carry multiple CspA paralogs with different expression kinetics, suggesting adaptation to both rapid chilling and prolonged cold periods.
Desaturase upregulation for membrane fluidity maintenance is the second pathway we target in NB-002, our cold-stress candidate currently in AI screening. Specifically, we look for the capacity to upregulate delta-9 fatty acid desaturase activity in response to temperature downshift, which introduces double bonds into membrane fatty acid chains and maintains bilayer fluidity at temperatures where saturated lipids would begin to crystallize. The genomic signal for this is present in several of our psychrotolerant Actinobacterial isolates from high-altitude steppe collection sites.
Cryoprotectant production is the third mechanism of interest. Several psychrotolerant bacteria produce compounds that function similarly to antifreeze proteins in fish: they bind to ice crystal surfaces and inhibit crystal growth, reducing the size and sharpness of extracellular ice crystals that form during a frost event. Bacterial ice crystal inhibition is not as potent as plant antifreeze proteins in terms of thermal hysteresis, but even modest reductions in crystal size can reduce membrane puncture damage during the frost-thaw cycle.
How Cold-Stress Bacteria Might Help the Crop
The mechanisms through which a psychrotolerant rhizobacterium could reduce cold damage to a crop plant are less direct than they are for salinity. The bacterium is in the soil; the frost damage happens primarily in the shoot tissue above ground. The link requires that root colonization induces systemic responses in the plant that change shoot cold tolerance, rather than a direct physical interaction at the site of damage.
There is published evidence for this type of induced systemic tolerance (IST). Root colonization by certain cold-adapted rhizobacteria has been shown to induce the expression of cold-responsive genes in shoot tissue, including CBF transcription factors that regulate the cold acclimation response in Arabidopsis and related cold-tolerance pathways in crop species. The mechanism involves systemic signaling, probably jasmonate-mediated, that propagates information about rhizosphere conditions to the whole plant. Whether this effect is robust enough under field conditions on Patagonian farmland to measurably reduce frost damage in maize or potato seedlings is what we need to test, and it is why NB-002 is in AI screening rather than field trial: we need better genomic and biochemical evidence for the IST pathway before we invest in the field trial infrastructure.
The Crop Varieties That Are Most Exposed
Not all crops in Patagonian growing regions face equivalent frost exposure risk. Maize is the most frost-vulnerable major grain in this context: it is a C4 crop with tropical evolutionary origins, and it has very low tolerance for temperatures below 10C during early vegetative development, with hard frost events at emergence being potentially lethal. Potato is a different profile: it has Andean evolutionary origins and somewhat higher chilling tolerance in vegetative tissue, but its tuber initiation period is highly frost-sensitive and a late frost during that developmental window can eliminate tuber yield even if the foliage recovers.
Chickpea and lentil, which are our target crops for NB-003, occupy a different cold-stress risk space. They are cool-season legumes with considerably higher intrinsic chilling tolerance than maize, but they are grown in semi-arid conditions in Patagonian valleys where water is limiting and the combination of cold nights, saline soil, and drought creates a multi-stress scenario that single-mechanism inputs cannot address. The rationale for NB-003's dual salinity-drought focus reflects exactly this situation.
Where Our Confidence Ends
We should be direct about what we do not know yet. We have promising isolates with relevant genomic profiles. We have published evidence from other research groups that the IST pathway from rhizobacteria to shoot cold tolerance is real under controlled conditions. What we do not have yet is our own demonstration that any of our Patagonian isolates produce a measurable reduction in cold damage to maize or potato under the specific temperature profiles of a Patagonian spring frost. That demonstration requires cold-chamber assays with the isolates under the right temperature protocols, followed by greenhouse trials with controlled frost events, before a field trial is justified.
We are working toward that evidence. We are not claiming it exists before we have generated it. The mechanism is credible, the genomic basis is present in the strains we are screening, and the agronomic need is real. That combination justifies continued investment in NB-002 through the AI screening and into phenotypic validation. It does not justify claiming a product effect we have not measured.